Review and Progress
Alternate Bearing Patterns and Supporting Cultivation Management in Torreya grandis 

2 Zhejiang Agronomist College, Hangzhou, 310021, Zhejiang, China
 Author Correspondence author
Plant Gene and Trait, 2026, Vol. 17, No. 5
Received: 27 Aug., 2026 Accepted: 30 Sep., 2026 Published: 12 Oct., 2026
Torreya grandis is an important woody oil-bearing and specialty economic forest species in China. However, alternate bearing occurs to varying degrees in production and has a substantial impact on yield stability, seed quality, and the sustainable management of orchards. This review summarizes the alternate-bearing characteristics of T. grandis and the corresponding cultivation management strategies, with particular emphasis on the effects of crop load, tree nutrient depletion, flower-bud formation, changes in tree vigor, environmental conditions, and cultivation practices on the development of alternate bearing. Studies in other perennial fruit crops indicate that heavy crop load creates strong reproductive sinks and may inhibit subsequent flowering through resource competition and hormonal regulation; the relative contribution of these processes in T. grandis remains to be established. By contrast, the reduced reproductive burden during off-years facilitates the recovery of shoots, roots, and nutrient reserves. Repeated alternation between on-years and off-years may further affect fruiting-branch renewal, tree nutrient cycling, and continuous fruiting capacity. To alleviate these effects, crop load should be regulated through appropriate fruit thinning, fruiting branches should be renewed through training and pruning, and moderate irrigation, stage-specific fertilization, and soil fertility improvement should be implemented according to tree vigor and bearing status. In addition, differential management between on-years and off-years and a dynamic tree-vigor monitoring system should be established. Future research should strengthen long-term continuous monitoring of alternate bearing in T. grandis, determine appropriate crop-load thresholds and nutrient recovery standards, and integrate physiological indicators, molecular regulation, rootstock selection, and digital monitoring technologies to develop precision stable-yield cultivation systems suitable for different tree ages and production regions. These efforts may provide a theoretical basis and technical reference for reducing annual yield fluctuations, maintaining tree health, and improving the long-term stability of the T. grandis industry.
1 Introduction
Torreya grandis is a relict evergreen conifer endemic to China and an important woody oil-bearing and specialty economic forest species with considerable economic, ecological, and cultural value. Its seeds can be used in food products, edible oils, medicinal products, and other value-added applications, giving the species substantial cultivation and utilization value in subtropical regions of China (Chen and Jin, 2019; Han et al., 2021). At present, natural populations and cultivated stands of T. grandis are mainly distributed in the middle and northern subtropical regions of eastern and southeastern China, where warm and humid climatic conditions and fertile acidic soils favor normal growth and fruiting. T. grandis has a long growth cycle and economic lifespan, and overall tree growth is relatively slow. Vegetative growth is comparatively rapid before approximately 45 years of age and gradually slows as trees become older. In terms of annual growth rhythm, shoots and other organs generally exhibit a distinct “slow-fast-slow” pattern, with the most vigorous growth occurring in spring and summer (Ma et al., 2023; Chen et al., 2024). As tree age increases, the crown gradually expands and branch complexity increases, while fruiting capacity becomes increasingly influenced by branch age, branch vigor, and the canopy light environment. Studies have shown that T. grandis seedlings are sensitive to light conditions, and moderate shading can increase height increment, basal diameter increment, biomass accumulation, and photosynthetic capacity, indicating that the canopy microenvironment can influence subsequent fruiting potential through its effects on vegetative growth and tree vigor (Tang et al., 2015). Therefore, an appropriate canopy structure, continuous branch renewal, and sufficient effective leaf area are important prerequisites for maintaining long-term and stable fruiting in T. grandis.
Seed development in T. grandis extends across two calendar years and generally lasts approximately 16~17 months, depending on the developmental stage used to define the starting point. Fruit growth generally follows an S-shaped pattern: enlargement is relatively slow from early summer to winter, changes little during winter, accelerates from the following spring to midsummer, and gradually reaches maturity after August (Zhang and Xiao, 2011). This prolonged fruit-development period causes considerable temporal overlap between current fruit enlargement and shoot renewal, leaf formation, and the initiation of the next reproductive cycle. Consequently, photosynthates produced by the canopy and mineral nutrients absorbed by the roots must be continuously allocated among shoot and leaf growth, root renewal, fruit development, and reproductive-organ formation. When crop load is moderate, vegetative and reproductive growth can remain relatively balanced. Under excessive crop load, however, large amounts of resources are diverted to developing fruits, restricting shoot renewal and the accumulation of nutrient reserves within the tree. Fruit size in T. grandis is also jointly affected by nutrient supply, genetic background, and the canopy microenvironment, and differences in fruit volume among individual trees cannot be explained solely by tree size (Chen and Chen, 2020). These characteristics indicate that fruiting in T. grandis is strongly crop-load dependent. The fruiting status of the current year therefore influences not only current-season yield and seed quality but may also exert prolonged effects on subsequent growth and future reproductive performance through changes in nutrient accumulation and shoot development.
Alternate bearing is a typical form of cyclical yield fluctuation in perennial fruit trees, generally characterized by a high-yielding year followed by a substantial decline in production in the subsequent year, sometimes approaching complete crop failure. Pronounced year-to-year variation in fruiting also occurs in T. grandis, with substantial differences among consecutive years in flowering intensity, fruit set, and final yield. During an on-year, a larger proportion of fruiting branches carry crops, and both crop load per tree and total yield increase markedly. During an off-year, flowering intensity, fruit set, the proportion of effective fruiting branches, and yield per tree may all decline. In perennial fruit trees, on-years are often accompanied by smaller fruit, reduced fruit quality, and intensified competition between vegetative and reproductive growth, whereas off-years directly reduce orchard profitability because of insufficient production (Carraro et al., 2026). Such annual fluctuations are jointly influenced by tree age, tree vigor, crop load, and site conditions. The extent of annual yield fluctuation can also vary with pollination system and environmental conditions (Garcia et al., 2021). T. grandis is slow growing, has a long fruiting cycle, and is commonly propagated by grafting in commercial production; consequently, stable fruiting is continuously influenced by tree nutrient status, canopy light conditions, and reproductive load (Chen and Jin, 2019; Hu et al., 2024). In addition, T. grandis is dioecious, and natural pollination can be constrained by asynchronous maturation of male and female reproductive organs and by pollen vitality, while local environmental conditions and management practices may further amplify year-to-year variation in fruiting (Ma et al., 2023). In production, trees with weak vigor, insufficient branch renewal, or long-term inadequate management generally show more pronounced alternate bearing, whereas trees with favorable nutritional status, well-structured canopies, and relatively balanced crop loads tend to exhibit smaller annual yield fluctuations. Previous studies have also demonstrated that yield and fruit quality in T. grandis are closely associated with nutrient supply and cultivation conditions. Excessive fertilization does not necessarily improve growth or yield, whereas moderate and balanced nutrient supply is more conducive to maintaining coordinated vegetative growth and fruiting (Han et al., 2021; Ma et al., 2023). Studies of other alternate-bearing fruit trees likewise indicate that crop load, nutrient status, canopy light interception, pruning, irrigation, and fertilization can all influence the intensity of alternate bearing (Krasniqi et al., 2017; Jangid et al., 2023).
Alternate bearing in T. grandis should not be regarded simply as a difference in yield between successive years, but rather as the integrated outcome of long-term interactions among nutrient allocation, shoot renewal, reproductive development, canopy environment, and cultivation management. Clarifying the relationships among tree growth, crop load, and resource allocation during alternate-bearing cycles is fundamental to understanding long-term yield fluctuations in T. grandis. Accordingly, this study systematically analyzes the formation patterns and major factors associated with alternate bearing in T. grandis, with particular emphasis on the interactions among tree age and vigor, vegetative and reproductive growth, crop load, canopy structure, nutrient supply, and cultivation management. The aim is to further elucidate the physiological and cultivation-related basis of alternate bearing and to provide a theoretical foundation and practical reference for optimizing tree management, balancing annual crop load, reducing yield fluctuations, and developing a high-quality, stable-yield cultivation management system for T. grandis.
2 Main Causes of Alternate Bearing in Torreya grandis
2.1 Fruit load and tree nutrient depletion
The occurrence of alternate bearing in Torreya grandis is closely associated with annual crop load and the allocation of tree resources. In perennial fruit trees, developing fruits during an on-year act as strong reproductive sinks and continuously compete for photosynthates produced by leaves and mineral nutrients absorbed by roots. As a result, carbohydrates, nitrogen, phosphorus, potassium, and other resources are preferentially allocated to fruit growth and seed-kernel formation, while fewer resources remain available for shoot renewal, root growth, flower-bud formation, and reserve accumulation. Previous studies have identified reduced return bloom after heavy cropping as a major feature of alternate bearing. Its physiological basis mainly involves two interacting processes: resource competition and fruit-derived hormonal regulation. Developing fruits may reduce the resource basis for floral induction by consuming carbohydrates and mineral nutrients, while gibberellin-related and other hormonal signals may further inhibit the transition of buds toward reproductive development (Campbell and Kalcsits, 2024; Carraro et al., 2026). Similar processes may be relevant to T. grandis, although direct mechanistic evidence is limited. Its fruit-development period lasts approximately 16 months and spans two calendar years, resulting in prolonged temporal overlap between current fruit growth and the accumulation of nutrients and flower-bud formation for the next reproductive cycle (Zhang and Xiao, 2011). This prolonged developmental overlap may intensify competition between fruit development, shoot renewal, and reserve accumulation during heavily cropping years.
Tree nutrient depletion further amplifies the effects of high crop load. Nutrient allocation differs markedly among organs in T. grandis, with leaves containing relatively high nitrogen concentrations, while the proportional distribution of elements among organs also changes with tree age. This indicates that tree nutritional status is dynamic and cannot be assessed solely on the basis of a single element or tissue (Chen et al., 2024). Appropriate nitrogen, phosphorus, and potassium supply can promote sapling growth, biomass accumulation, and nutrient allocation to leaves and roots (Ma et al., 2023), but increasing fertilizer input does not necessarily compensate fully for the resource depletion associated with an on-year. Under conditions of high atmospheric nitrogen deposition in subtropical regions, long-term heavy fertilization in mature T. grandis orchards did not effectively increase carbon accumulation, tree growth, or seed yield, while excessive nitrogen input could disturb plant C stoichiometric balance (Han et al., 2021). These findings suggest that alternate bearing in T. grandis is not simply caused by “insufficient fertilization”; rather, the key issue lies in whether crop load is properly matched with nutrient supply, uptake, and storage capacity.
The nutritional imbalance created during an on-year also has a clear carry-over effect across years. When heavy cropping continuously depletes tree reserves, insufficient postharvest recovery weakens the material basis for shoot growth and flower-bud formation in the following year, resulting in reduced flowering and fruiting. By contrast, during an off-year, the lower fruit number reduces competition from reproductive sinks, allowing more assimilates to be redirected toward vegetative growth and reserve storage, thereby rebuilding the capacity for stronger fruiting in subsequent years (Jangid et al., 2023; Carraro et al., 2026). These findings suggest that interactions among crop load, resource depletion, floral induction, and subsequent nutrient recovery may contribute to alternate bearing in T. grandis. However, the underlying physiological mechanisms require further validation through long-term studies of tree nutrient reserves, hormonal regulation, and flowering dynamics.
2.2 Flower-bud formation and changes in tree vigor
Flower-bud formation is a critical link between current-season tree growth and yield in the following year, and it represents a key developmental stage in the transition from heavy cropping in an on-year to low yield in the subsequent off-year. Stable year-to-year fruiting in perennial fruit trees depends largely on the maintenance of normal floral induction and differentiation each season (Sharma et al., 2019). During an on-year, when fruit number is high, developing fruits, new shoots, and flower buds compete simultaneously for carbohydrates and mineral nutrients. Consequently, some fruiting branches may show reduced shoot extension, insufficient tissue maturation, and suppressed flower-bud formation. In addition to resource competition, hormonal signals generated or regulated by developing fruits may also participate in floral inhibition, with gibberellin-related pathways considered especially important in the regulation of alternate bearing in perennial fruit trees (Krasniqi et al., 2017; Campbell and Kalcsits, 2024; Carraro et al., 2026). Therefore, the negative effect of an on-year on the following season’s fruiting capacity cannot be explained simply as a consequence of “reduced tree nutrients,” but rather as the combined outcome of resource limitation and reproductive-developmental regulation.
The intrinsic growth characteristics of T. grandis further influence these processes. Overall tree growth is relatively slow, and tree height and diameter at breast height exhibit distinct age-related developmental stages, with comparatively rapid growth before approximately 45 years of age and a gradual decline thereafter. Element allocation patterns also differ among trees of different ages (Chen et al., 2024). These characteristics imply that branch renewal and the capacity of trees to buffer heavy reproductive demand may change with age. In weak trees, repeated heavy cropping is more likely to result in insufficient shoot renewal and a reduced proportion of effective fruiting branches. During an off-year, by contrast, the lower reproductive burden allows vegetative growth and reserve accumulation to recover, thereby rebuilding the material basis for flower-bud formation in the following year. However, excessively vigorous vegetative growth during an off-year may also lead to shoot overgrowth and canopy crowding, thereby reducing effective light interception and potentially impairing stable floral induction. Thus, stable fruiting does not simply depend on maintaining high tree vigor, but rather on preserving a relatively balanced relationship between vegetative and reproductive growth.
The reproductive biology of T. grandis may further increase year-to-year uncertainty in fruiting. T. grandis is dioecious, and natural pollination is influenced by asynchronous maturation of male and female reproductive organs as well as pollen vitality. Pollen germination and pollen-tube growth also respond markedly to external environmental conditions (Hu et al., 2024). When flowering has already declined following an on-year, additional constraints such as poor flowering synchrony, low pollen vitality, or unfavorable weather may further reduce fruit set. Therefore, flower-bud formation, maintenance of tree vigor, pollination, and fertilization should not be regarded as isolated processes, but rather as interconnected components of the continuous reproductive process from flowering to final fruit set in T. grandis.
2.3 Effects of environmental conditions and cultivation management
Environmental conditions can directly affect flowering, pollination, fruit set, and fruit development in T. grandis, while also modifying the intensity of alternate bearing through their effects on tree growth and nutritional status. In perennial fruit trees, external factors such as low temperature, frost, abnormal heat, changes in rainfall, water stress, pests, and diseases can induce or amplify year-to-year yield fluctuations (Krasniqi et al., 2017; Garcia et al., 2021; Jangid et al., 2023). T. grandis has a relatively well-defined ecological adaptation range, with its natural distribution concentrated mainly in the middle and northern subtropical regions of China. The species is generally associated with warm, humid subtropical conditions and suitable well-drained soils (Chen and Jin, 2019). Microclimatic differences associated with elevation, slope aspect, solar radiation, wind exposure, and extreme low temperatures can also influence growth and fruiting performance. Consequently, the intensity of alternate bearing may differ among orchards even within the same production region, because long-term site conditions can affect tree vigor, flowering, and fruit set.
The light environment is another important factor affecting tree vigor in T. grandis. Tang et al. (2015) investigated the growth and photosynthetic responses of T. grandis seedlings under different shading treatments and found that moderate shading promoted height growth, basal diameter increment, biomass accumulation, and photosynthetic performance, whereas both full sunlight and excessive shading could inhibit growth. Although seedling responses to light cannot be directly equated with alternate-bearing patterns in mature fruiting trees, these findings indicate that T. grandis is highly responsive to canopy light conditions. In mature orchards, long-term lack of appropriate pruning can result in canopy crowding and insufficient light penetration into the inner canopy, thereby reducing photosynthate production and limiting the renewal of fruiting branches. Fruit size and commercial value are also influenced by tree nutritional status, crop load, and canopy microenvironment (Figure 1) (Chen and Chen, 2020). Thus, site conditions and canopy environment together constitute important external determinants of alternate-bearing expression.
 Figure 1 Fruits of Chinese torreya (Adopted from Chen and Chen, 2020) |
Cultivation management can further amplify or buffer these environmental effects. Long-term lack of appropriate pruning can lead to canopy crowding, aging fruiting wood, and a decline in effective fruiting sites. Failure to regulate crop load during an on-year can further increase tree resource depletion, whereas inappropriate fertilizer timing, type, or application rate may create a mismatch between nutrient supply, fruit development, and tree recovery. Importantly, higher fertilizer input is not necessarily more beneficial in mature T. grandis orchards; prolonged excessive nitrogen fertilization may disturb nutrient balance without producing corresponding gains in growth or yield (Han et al., 2021). Studies in other perennial fruit crops likewise show that pruning, thinning, irrigation, fertilization, and flowering-stage management can influence the intensity of alternate bearing by modifying crop load, tree nutritional status, and floral induction (Krasniqi et al., 2017; Jangid et al., 2023). Therefore, alternate bearing in T. grandis should be understood as a continuous feedback process jointly shaped by crop load, nutrient allocation, tree vigor, flower-bud formation, ecological conditions, and cultivation management, rather than as an annual yield fluctuation caused by any single factor.
3 Changes in Tree Growth and Yield of Torreya grandis under Alternate Bearing
3.1 Tree growth and nutrient depletion in on-years
Once Torreya grandis enters an on-year, the high crop load markedly alters the internal pattern of resource allocation. A greater proportion of limited assimilates and mineral nutrients is directed toward fruit development and seed-kernel formation, while fewer resources remain available for shoot elongation, branch thickening, root renewal, and reserve accumulation. In perennial fruit trees, the strong sink effect generated by a high reproductive load generally suppresses vegetative growth and reduces non-structural carbohydrate reserves in roots, stems, and shoots (Shalom et al., 2012; Khezri et al., 2020; Carraro et al., 2026). This feature is particularly important in T. grandis. The species grows relatively slowly and has a prolonged fruit-development period, so sustained fruit growth during an on-year can compete with canopy renewal and reserve accumulation for an extended period. Studies on T. grandis have also shown that nitrogen, phosphorus, and potassium supply can significantly influence sapling growth and nutrient allocation among organs, indicating that tree growth depends strongly on the balance between nutrient supply and demand (Ma et al., 2023).
The effects of heavy crop load are not limited to weakened shoot growth during the current season but also extend to reduced postharvest reserve levels. In mature pistachio trees, on-year trees stored significantly less nitrogen, phosphorus, and potassium than lightly cropping trees and relied more heavily on nutrient resorption from senescing leaves to sustain fruit development (Rosecrance et al., 1998). Isotopic studies further showed that on-year pistachio trees lost approximately five times more nitrogen through fruits and senescent leaves than off-year trees and entered dormancy with markedly lower starch and nitrogen reserves (Weinbaum et al., 1994). Together, these findings indicate that high production in an on-year is often achieved at the cost of substantial tree resource depletion.
For T. grandis, weakened shoots, reduced renewal capacity, and slow recovery of tree vigor after an on-year cannot simply be corrected by increasing fertilizer input. Studies in mature T. grandis orchards have shown that under conditions of high nitrogen deposition, additional nitrogen fertilization did not effectively promote carbon accumulation, tree growth, or seed yield and could instead disturb plant nutrient stoichiometric balance (Han et al., 2021). Therefore, the effects of an on-year on the tree are essentially the combined result of crop load, nutrient uptake, and internal resource redistribution. If heavy cropping persists over consecutive years, trees may gradually exhibit poorer branch maturation, aging fruiting wood, and insufficient nutrient reserves, creating a clear conflict between high current-year yield and the long-term maintenance of tree vigor.
3.2 Tree recovery and nutrient accumulation in off-years
Compared with an on-year, the decline in crop load during an off-year markedly reduces competition from fruits for assimilates and mineral nutrients, allowing more resources to be allocated to the recovery of shoots, leaves, roots, and perennial tissues. In typical alternate-bearing fruit trees, off-years are generally characterized by stronger vegetative growth and renewed accumulation of non-structural carbohydrates (Shalom et al., 2012; Carraro et al., 2026). Studies in citrus have shown that off-year trees exhibit distinct peaks in root growth and may produce multiple vegetative shoot flushes, whereas root activity is strongly suppressed in on-year trees (Stander et al., 2018). Therefore, for T. grandis trees weakened by heavy cropping in the previous year, the off-year represents not merely a period of lower yield but an important phase for readjusting resource allocation and restoring shoot and root vigor.
Another major feature of off-year recovery is the replenishment of stored nutrients. In pistachio, overall carbohydrate levels are higher in off-year trees than in on-year trees, and reduced crop load allows reserve materials to accumulate again in roots, stems, and branches (Guney et al., 2023). Weinbaum et al. (1994) further reported that pistachio trees entering dormancy after an off-year contained 144% more starch and 22% more nitrogen reserves than trees after an on-year, while uptake of labeled nitrogen was approximately 60% greater. Rosecrance et al. (1998) also found that lightly cropping trees stored about 7, 14, and 2 times as much N, P, and K, respectively, as heavily cropping trees. These findings indicate that an off-year not only reduces competition from developing fruits but also provides greater opportunity for the tree to absorb, redistribute, and store nutrients.
Research on nutrient cycling in T. grandis provides additional support for this interpretation. Fan et al. (2025) found that nutrient-cycling patterns among leaves, litter, and soil changed markedly with stand development, nitrogen resorption efficiency increased during mature and overmature stages, and soil nutrient accumulation generally increased with stand age; tree age and soil nutrient supply also influenced seed quality. These findings indicate that T. grandis has strong perennial nutrient-cycling and reutilization characteristics. Whether leaf function, shoot growth, and nutrient reserves can be effectively restored during an off-year is therefore likely to be important for rebuilding reproductive capacity in the following season. However, stronger vegetative growth during an off-year is not always beneficial. Excessive shoot growth may lead to canopy crowding, thereby reducing effective light interception and fruiting-branch quality. Thus, off-year management should emphasize physiological recovery rather than simply promoting vigorous vegetative growth.
3.3 Effects of on-year and off-year alternation on continuous fruiting capacity
The continuous fruiting capacity of T. grandis depends on whether the tree can complete current fruit development while maintaining sufficient shoot renewal, nutrient reserves, and the physiological basis for floral initiation in the following year. Repeated alternation between on-years and off-years continuously alters this balance. In perennial fruit trees, on-years are generally associated with greater resource depletion and weaker return bloom, whereas off-years reduce reproductive load and thereby provide conditions favorable for nutrient recovery and renewed flower-bud formation (Sharma et al., 2019; Carraro et al., 2026). Such recovery is not necessarily completed within a single growth cycle. In some species, one heavy-cropping year may be followed by several low-yield years, indicating that the physiological after-effects of an on-year can persist beyond the following season (Shalom et al., 2012). Continuous fruiting capacity therefore depends on whether a relatively stable dynamic balance can be maintained among current-year yield, tree resource depletion, the degree of recovery, and flower formation in the subsequent year.
For T. grandis, this issue should be evaluated over a multi-year timescale. The species is long-lived and has an extended fruiting lifespan, while stands of different ages also exhibit distinct nutrient limitations and resorption strategies. Fan et al. (2025) studied T. grandis stands aged 20, 50, 80, 100, and 1 000 years and found that young stands were primarily limited by nitrogen, whereas phosphorus limitation became more pronounced with increasing stand age. Nitrogen resorption efficiency increased in mature and overmature stages, and seed nutritional quality was also influenced by tree age and nutrient-use characteristics. Therefore, if alternate bearing remains unmanaged over long periods, repeated excessive depletion during on-years combined with insufficient recovery during off-years may gradually impair fruiting-branch renewal, nutrient cycling, and yield efficiency per unit canopy. Evaluating orchard performance solely on the basis of a single high-yielding year may therefore overlook negative effects on tree condition in the following year and over longer periods. Assessment of stable production in T. grandis should consequently shift from single-year yield toward an integrated evaluation of multi-year yield, return bloom, shoot renewal, and tree nutritional status.
4 Supporting Cultivation Measures for Regulating Alternate Bearing in Torreya grandis
4.1 Fruit load regulation and proper fruit thinning
Fruit load regulation may provide a direct approach to alleviating alternate bearing in Torreya grandis, but species-specific thinning thresholds have not yet been established. During an on-year, excessive fruit load creates a strong reproductive sink that continuously competes for photosynthates and mineral nutrients and, through both resource depletion and fruit-derived hormonal signals, suppresses floral induction and return bloom in the following year. Therefore, appropriately reducing crop load is an important means of restoring the balance between vegetative and reproductive growth (Fichtner et al., 2021; Jangid et al., 2023; Carraro et al., 2026). This measure is particularly important for T. grandis because its prolonged fruit-development period extends the duration of source–sink competition under heavy cropping. When fruit set markedly exceeds the carrying capacity of the tree, shoot growth and reserve accumulation may decline, while the risks of producing undersized fruit and reduced fruit quality may increase. Accordingly, on-year thinning trials should evaluate fruit retention in relation to tree age, vigor, crown size, fruiting-branch proportion, and fruit set. Priority should be given to removing excessively clustered, weak, malformed, or poorly positioned fruits so that the remaining crop is distributed more evenly throughout the canopy.
The timing of fruit thinning also affects its regulatory effectiveness. Studies on perennial fruit trees generally show that early crop-load reduction is more effective than corrective thinning later in fruit development because early removal reduces sink strength before large amounts of carbohydrates and mineral nutrients are irreversibly allocated to developing fruits. In apple, crop-load regulation after flowering and during early fruit development improved individual fruit weight, fruit size, and return bloom in the following year, with more pronounced improvements in return bloom when flower-cluster load was reduced to a greater extent (Netsawang et al., 2023). In olive, reducing fruit load within approximately 120 days after full bloom still significantly restored vegetative growth and return bloom in the following season (Dag et al., 2010). These interspecific findings suggest testing relatively early thinning in T. grandis during on-years, with the protection of next-year fruiting potential regarded as an important objective rather than focusing solely on current-year fruit size and yield.
Fruit-thinning management should also avoid the use of a completely fixed fruit-retention standard and instead be adjusted dynamically according to tree condition. Trees with strong vigor, sufficient leaf area, and a well-balanced branch structure may be able to maintain a relatively high crop load, whereas weak trees, trees with insufficient branch renewal, or trees that have previously carried excessive crops should retain fewer fruits. During off-years, excessive efforts to maximize fruit set should likewise be avoided, as this may simply recreate excessive resource depletion in the subsequent year. Continuous observation of flowering intensity, fruit set, shoot growth, and tree recovery can help establish a crop load that is better matched to tree vigor, thereby shifting T. grandis production away from the pursuit of maximum single-year yield toward a balance between current returns and multi-year yield stability.
4.2 Training, pruning, and renewal of fruiting branches
The primary role of training and pruning is to improve canopy structure, enhance ventilation and light penetration, and continuously maintain an adequate proportion of vigorous vegetative and renewal shoots. In perennial fruit trees with alternate bearing, pruning cannot directly eliminate the physiological basis of biennial yield fluctuation, but it can buffer the suppressive effects of an on-year on subsequent flowering by changing the ratio of fruiting to vegetative shoots, improving canopy light-use efficiency, and promoting the formation of new shoots (Lazare et al., 2021). Long-term stable production in T. grandis likewise depends on maintaining a dynamic balance between healthy fruiting wood and renewal shoots. Therefore, mature trees should be managed by selectively removing crossing, overlapping, weak, and senescent branches to prevent localized canopy crowding, while moderate heading-back should be used to renew aging fruiting units so that newly formed shoots can gradually assume future fruiting functions.
Pruning method and intensity should be coordinated with on-year and off-year conditions. On-year trees carry a heavier reproductive burden and should therefore not be subjected to excessive pruning. Management should focus on removing ineffective branches, improving internal canopy light conditions, and reducing localized crop load while avoiding further weakening of tree vigor. In off-years, when reproductive pressure is lower, somewhat stronger renewal of fruiting units and canopy restructuring can be used to develop vigorous fruiting shoots for the following season. Available evidence generally supports continuous and moderate renewal pruning rather than severe pruning at long intervals. In ‘Nadorcott’ mandarin, annual half-length pruning promoted summer and autumn shoot formation, increased readiness for floral induction, raised cumulative yield by 25% over four years, and reduced alternate-bearing intensity (Mesejo et al., 2020). Studies in jojoba also showed that top pruning effectively promoted new shoot formation and yield recovery, while several pruning strategies reduced alternate-bearing cycles to varying degrees (Lazare et al., 2021).
Research in other fruit crops further indicates that pruning response is closely related to crop load in the preceding year. In peach, previous-year fruit density was an important trigger of alternate bearing, whereas lighter winter pruning helped maintain yield when return bloom was weak (Bussi and Génard, 2014). Therefore, training and pruning in T. grandis should move beyond simply controlling tree shape and instead adopt coordinated regulation of “canopy structure-branch age-crop load.” Through continuous renewal of fruiting branches, appropriate proportions of vegetative, fruiting, and renewal shoots can be maintained, thereby reducing the amplification of alternate bearing caused by branch aging and outward migration of fruiting sites.
4.3 Water and fertilizer regulation and tree nutrient management
Water and fertilizer management form an important foundation for maintaining tree vigor, supporting fruit development, and buffering year-to-year yield fluctuations in T. grandis. The central principle should be to match resource supply with tree demand rather than maximize input. Studies on perennial fruit trees show that both nutrient deficiency and excessive fertilization can intensify alternate bearing. In olive, prolonged low nitrogen supply reduced vegetative growth, flowering intensity, fruit set, and yield and increased susceptibility to alternate bearing, whereas excessive nitrogen stimulated shoot and leaf growth without a corresponding increase in yield. By contrast, intermediate nitrogen supply produced better long-term production stability (Haberman et al., 2019). Therefore, water and fertilizer management during an on-year in T. grandis should aim to meet the requirements of fruit development while supporting tree recovery. Nutrient shortages during fruiting should be avoided, but heavy crop-load depletion should not simply be compensated for by increasing nitrogen input.
Research on T. grandis itself also supports a balanced fertilization strategy. Appropriate N, P, and K supply can promote sapling height growth, basal diameter increment, biomass accumulation, and nutrient accumulation in different organs, with nitrogen playing a particularly important role in nutrient accumulation (Ma et al., 2023). However, under conditions of high nitrogen deposition in subtropical regions, excessive nitrogen addition in mature T. grandis orchards did not effectively improve carbon accumulation, tree growth, or seed yield and could instead disturb nutrient stoichiometric balance (Table 1) (Han et al., 2021). These findings indicate that water and fertilizer management should be adjusted according to tree age, crop load, soil fertility, and leaf nutrient status. During the early and middle stages of an on-year, water and mineral nutrient supply should primarily support fruit development, while postharvest management should emphasize reserve restoration. During an off-year, although crop load is lower, fertilization should not simply be discontinued; instead, moderate nutrient supply should be maintained while excessive nitrogen application that could induce overly vigorous shoot growth should be avoided.
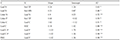 Table 1 Relationships of nutrients among soil, leaves, and litter through SMA analyses (Adopted from Han et al., 2021) Table caption: * and ** are 2-tail sig. p<0.1 and 0.05; TP: Total Phosphorus; HN: Hydrolyzable Nitrogen; SOC: Soil Organic Carbon; PRE: Phosphorus Resorption Efficiency; SMA: Standardized Major Axis analysis (Adopted from Han et al., 2021) |
Water management should be coordinated with fertilization. If prolonged drought occurs during flowering, early fruit development, or fruit enlargement, timely irrigation is required to maintain root uptake and leaf photosynthetic function. During the rainy season or in low-lying orchards, drainage should be strengthened to prevent prolonged waterlogging from reducing root activity. Soil improvement is also important in T. grandis orchards. Under simulated nitrogen deposition, biochar application increased soil pH and the availability of N, P, and K while improving seed weight and nutritional quality in T. grandis (Zhang et al., 2017). Therefore, water and fertilizer regulation for alternate-bearing control in T. grandis should follow the basic principles of “moderate irrigation-stage-specific fertilization-soil fertility improvement-avoidance of excessive nitrogen input.” By improving water-and nutrient-use efficiency and strengthening tree recovery, this approach can help prevent excessive depletion during on-years and promote reserve restoration during off-years, thereby supporting more continuous and stable production.
5 Development of a Stable-Yield Cultivation Management System for Torreya grandis
5.1 Differential management of on-years and off-years
Management of alternate bearing in Torreya grandis should not follow an identical annual strategy but should instead be adjusted according to flowering intensity, fruit set, crop load, and tree vigor in a given year. During on-years, management should focus on reducing excessive crop load, protecting tree reserves, and maintaining return bloom in the following season. Studies on perennial fruit trees have shown that heavy crop load suppresses summer shoot growth, increases flower-bud loss, interferes with physiological processes related to floral development, and reduces spring bud break and return bloom (Fichtner et al., 2021). Therefore, the management objective in an on-year should not simply be to maximize single-year yield. Rather, moderate fruit thinning, light pruning, and balanced water and nutrient supply should be used to maintain crop load within the carrying capacity of the tree. Early crop-load regulation is generally more effective than late corrective intervention because reducing excessive reproductive sinks shortly after flowering or during early fruit development can decrease unnecessary resource depletion while improving fruit size, return bloom, and annual yield stability (Netsawang et al., 2023). This management concept is particularly important for T. grandis because its prolonged fruit-development period means that heavy cropping can occupy tree resources for an extended time.
Management during off-years should shift from “crop-load control” toward “tree recovery, renewal of fruiting wood, and preservation of flowering potential”. Once reproductive pressure is reduced, more resources can be allocated to shoot growth, recovery of leaf function, and nutrient storage. However, if management inputs are substantially reduced during this period, an important opportunity for restoring tree vigor and preparing the following year’s crop may be lost. Direct studies of T. grandis emphasize balanced nutrient supply and the avoidance of excessive nitrogen inputs rather than fixed off-year fertilization formulas (Han et al., 2021; Fan et al., 2025). Therefore, off-year management in T. grandis should maintain an appropriate nutrient supply, promote the development of vigorous shoots and renewal of fruiting branches, and at the same time avoid excessive nitrogen application and overly vigorous shoot growth.
Management during on-years and off-years should also be linked across successive seasons rather than treated as two independent annual programs. Research on alternate-bearing fruit trees indicates that crop load and reserve recovery can influence subsequent flowering and production, although these carry-over effects have not yet been quantified in T. grandis (Carraro et al., 2026). Accordingly, stable-yield management in T. grandis should follow a continuous strategy of “controlling crop load and maintaining tree vigor during on-years, and promoting recovery and renewing fruiting wood during off-years,” thereby shifting the objective of orchard management from maximizing annual yield to maintaining multi-year balance.
5.2 Coordinated regulation of pruning, crop load, water, and fertilizer
The key to stable-yield management in T. grandis is to treat pruning, crop-load regulation, irrigation, and fertilization as an integrated and interdependent system rather than as separate practices. Alternate bearing is influenced not only by internal source-sink relationships and reproductive regulation but also by canopy conditions and external water and nutrient supply. Consequently, single-factor interventions often have limited capacity to stabilize yield over the long term (Jangid et al., 2023; Campbell and Kalcsits, 2024; Carraro et al., 2026). Pruning is primarily used to adjust canopy structure, improve light interception, and renew fruiting branches; fruit thinning directly determines current crop load and the degree of resource depletion; and water and fertilizer management provide the material basis for shoot and leaf growth, fruit development, and postharvest recovery. Only when these measures are properly coordinated can the balance between vegetative and reproductive growth be effectively improved.
Pruning and crop-load regulation, in particular, should be implemented in a coordinated manner. When the proportion of fruiting branches is too high and vegetative shoots are insufficient, tree vigor may decline because of excessive reproductive sink strength even if water and nutrients are adequately supplied. Conversely, when the canopy is overly dense or fruiting wood is senescent, thinning alone is unlikely to restore effective leaf area and subsequent flowering capacity. Studies in peach have shown that fruit density in the previous year is an important trigger of alternate bearing, while lighter winter pruning can help maintain yield when return bloom is weak (Bussi and Génard, 2014). In ‘Nadorcott’ mandarin, annual half-length pruning promoted summer and autumn shoot formation, enhanced readiness for floral induction, increased cumulative yield by approximately 25% over four years, and reduced alternate-bearing fluctuations (Mesejo et al., 2020). These findings indicate that the value of renewal pruning lies not only in controlling canopy size but also in maintaining a dynamic balance between fruiting and renewal shoots in combination with crop-load regulation.
Water and fertilizer management should be further integrated into this coordinated system. Appropriate irrigation supports root activity and leaf photosynthetic capacity, but water management alone cannot be assumed to resolve floral inhibition and source-sink competition (Carraro et al., 2026). Fertilization should likewise avoid the simple assumption that a heavier crop requires proportionally more fertilizer. Research in olive has shown that low nitrogen supply increases the risk of alternate bearing, whereas excessive nitrogen stimulates vegetative growth without a corresponding increase in yield; intermediate nitrogen supply instead provides better long-term yield stability (Haberman et al., 2019). Therefore, in T. grandis, pruning intensity, fruit retention, irrigation amount, and fertilizer input should be determined simultaneously according to tree vigor, crop load, and developmental stage so that canopy structure, reproductive load, and nutrient supply remain relatively coordinated.
5.3 Tree vigor monitoring and dynamic management
Establishing a stable production system for T. grandis also requires a gradual shift from experience-based management to dynamic management based on continuous monitoring of tree vigor and reproductive status. Even when crop load is maintained at a relatively appropriate level in a given year, return bloom may remain unstable if shoot recovery is insufficient, nutrient reserves are low, or canopy renewal is restricted (Campbell and Kalcsits, 2024). Therefore, orchard management should continuously monitor indicators such as current-season shoot length, branch diameter, leaf color and leaf abundance, the proportion of fruiting branches, flowering intensity, fruit set, and yield per tree. These indicators, together with visible tree condition and annual yield changes, can be used to determine whether a tree is in an overloaded, balanced, or recovering state. Research on stable apple production has shown that, where long-term data are available, crop-load thresholds can be established on the basis of target flower-cluster numbers and the proportion of non-fruiting spurs, thereby improving the predictability of return bloom in the following year (Krasniqi et al., 2017). This threshold-based management concept may also be valuable for T. grandis.
Monitoring of tree vigor should also be combined with tree age, rootstock, site conditions, and historical yield records. In other fruit trees, alternate-bearing tendencies differ among cultivars, rootstocks, and orchard environments, and rootstocks can affect fruiting behavior through nutrient uptake, water transport, and hormonal signaling (Jangid et al., 2023; Carraro et al., 2026). Therefore, the same pruning or fertilization program may not be suitable for all trees. Trees with short current-season shoots, weak branches, declining leaf color, and heavy crop load should be prioritized for crop-load reduction and recovery management. By contrast, trees showing excessive shoot growth and rapid canopy crowding during an off-year should receive stronger vegetative control and canopy adjustment through pruning.
The core of dynamic management is the establishment of continuous multi-year records rather than making decisions solely on the basis of a single high- or low-yielding season. By recording flowering intensity, fruit-set rate, yield, shoot growth, water and fertilizer inputs, and pruning practices at the individual-tree or orchard level, the alternate-bearing rhythm and changing trends of different trees can be identified progressively. At the orchard scale, trees can further be classified as “overloaded”, “balanced”, or “recovering”, with corresponding crop-load, pruning, and nutrient-management strategies developed for each category. Such a closed-loop management system of “monitoring-classification-regulation-evaluation-readjustment” can gradually shift T. grandis production from passive responses to alternate bearing toward active regulation of tree balance across consecutive years.
6 Summary and Prospects
Alternate bearing in Torreya grandis is a continuous fruiting phenomenon resulting from the combined effects of tree growth, crop load, nutrient allocation, and environmental conditions, and its essence lies in a cyclical imbalance between reproductive demand and tree recovery. During an on-year, heavy crop load creates a strong reproductive sink, causing carbohydrates and mineral nutrients to be preferentially allocated to developing fruits and consequently restricting shoot growth, renewal of fruiting branches, and reserve accumulation. Evidence from other perennial fruit crops suggests that fruit-related hormonal signals may contribute to floral inhibition and reduced return bloom. Whether similar regulatory mechanisms operate in T. grandis requires further investigation. During an off-year, the reduced reproductive burden favors the renewed accumulation of N, P, K, and non-structural carbohydrates and promotes the recovery of tree nutritional status and shoot growth. Tree age, tree vigor, the proportion of fruiting branches, flower-bud formation, rootstock, site conditions, and cultivation practices can also modify the intensity of alternate bearing. Therefore, alternate bearing in T. grandis should not be regarded simply as an alternation between high- and low-yielding years, but rather as a dynamic process arising from feedback interactions among tree physiology, environmental conditions, and cultivation management. Accordingly, evaluation should shift from single-year yield toward the overall stability of fruiting across consecutive years.
The primary value of supporting cultivation management for alternate bearing in T. grandis lies in regulating crop load, canopy structure, and water and nutrient supply to reduce excessive resource depletion during on-years while maintaining sufficient physiological capacity for flowering and fruiting in the following season. Studies on perennial fruit trees have shown that timely flower or fruit thinning can improve fruit size and marketability while enhancing return bloom, whereas moderate pruning can improve canopy light conditions, renew fruiting wood, and increase the proportion of shoots with flowering potential. Appropriate water and nutrient management also contributes to the maintenance of tree vigor and nutrient reserves. For T. grandis, on-year management should focus on controlling crop load, maintaining tree vigor, and promoting postharvest recovery, whereas off-year management should take advantage of the lower reproductive burden to promote branch renewal and reserve accumulation while avoiding excessive nitrogen application and overly vigorous vegetative growth. Coordinated regulation of thinning, pruning, irrigation, and fertilization may therefore be more effective for maintaining long-term vegetative–reproductive balance than reliance on any single practice. The objective of stable-yield management should also extend beyond maximizing production in a particular year to include multi-year average yield, seed quality, tree health, labor organization, and economic stability, thereby improving the long-term productivity and resilience of T. grandis orchards.
Future research on stable-yield cultivation of T. grandis should gradually move from descriptive observations toward mechanistic analysis, indicator-based evaluation, and precision regulation. Long-term continuous monitoring of alternate bearing in T. grandis remains relatively limited. Future studies should therefore quantify seasonal changes in non-structural carbohydrates, N, P, K, and major hormones in leaves, shoots, roots, and reproductive buds during different stages of on- and off-years and relate these variables to flower-bud differentiation, shoot growth, return bloom, and final yield. Particular attention should be given to identifying critical crop-load thresholds that begin to suppress return bloom and the nutritional recovery levels required during off-years to maintain normal fruiting in the following season. Meanwhile, multi-year field trials across different production regions, tree ages, and vigor classes should integrate indicators such as the alternate-bearing index, multi-year mean yield, return-bloom rate, renewal of shoots, proportion of effective fruiting branches, leaf nutrient status, and fruit quality to establish a dynamic system for evaluating and managing stable production. Rootstock selection, transcriptomic and metabolomic analyses, marker-assisted breeding, as well as digital technologies such as unmanned aerial vehicles, canopy image analysis, flower-density recognition, and soil and leaf nutrient sensing, also deserve further attention. These approaches could facilitate the transition of T. grandis cultivation from experience-based management toward more quantitative, dynamic, and precision-oriented production systems.
Conflict of Interest Disclosure
The author affirms that this research was conducted without any commercial or financial relationships that could be construed as a potential conflict of interest.
Bussi C., and Génard M., 2014, Thinning and pruning to overcome alternate bearing in peach trees, European Journal of Horticultural Science, 79(6): 313-317.
https://doi.org/10.1079/ejhs.2014/4999700
Campbell T., and Kalcsits L., 2024, Strategies to overcome biennial bearing in apple-a review, European Journal of Agronomy, 158: 127213.
https://doi.org/10.1016/j.eja.2024.127213
Carraro P., Naeem M.Y., Girardi F., Botton A., Varotto S., Ruperti B., and Bonghi C., 2026, A rootstock-centered perspective on the regulation of alternate bearing in fruit trees, Journal of Experimental Botany, 77(2): 267-281.
https://doi.org/10.1093/jxb/eraf460
Chen L., Liu N., Wan Z.B., Liu F.F., Cao L., Gao C., Sun N., and Liu C.G., 2024, The growth equation and element distribution of Torreya grandis in the Huangshan region of China, Forests, 15(1): 68.
https://doi.org/10.3390/f15010068
Chen X.W., and Chen X., 2020, Variation of fruit size and its frequency distribution in Chinese Torreya, International Journal of Fruit Science, 20(S3): S1445-S1457.
https://doi.org/10.1080/15538362.2020.1802395
Chen X.W., and Jin H.B., 2019, Review of cultivation and development of Chinese torreya in China, Forests, Trees and Livelihoods, 28(1): 68-78.
https://doi.org/10.1080/14728028.2018.1553690
Dag A., Bustan A., Avni A., Tzipori I., Lavee S., and Riov J., 2010, Timing of fruit removal affects concurrent vegetative growth and subsequent return bloom and yield in olive (Olea europaea L.), Scientia Horticulturae, 123(4): 469-472.
https://doi.org/10.1016/j.scienta.2009.11.014
Fan A., Jin S., Tan Y., Huan W., Chen W., Wang X., and Han Y., 2025, Nutrient recycling and utilization of Torreya grandis ‘Merrillii’ along an age gradient, Frontiers in Plant Science, 16: 1566140.
https://doi.org/10.3389/fpls.2025.1566140
Fichtner E.J., Chao Y.Y., Ferguson L., Verreynne J.S., Tang L., and Lovatt C.J., 2021, Repeating cycles of ON and OFF yields in alternate bearing olive, pistachio and citrus trees-different mechanisms, common solutions, Acta Horticulturae, 1315: 1-10.
https://doi.org/10.17660/ActaHortic.2021.1315.1
Garcia G., Re B., Orians C., and Crone E., 2021, By wind or wing: pollination syndromes and alternate bearing in horticultural systems, Philosophical Transactions of the Royal Society B: Biological Sciences, 376(1839): 20200371.
https://doi.org/10.1098/rstb.2020.0371
Guney M., Gundesli M.A., Guney M., Kafkas S., and Kafkas N.E., 2023, Exploring carbohydrate concentration fluctuations in pistachio (Pistacia vera L. cv Uzun) for deeper insights into alternate bearing patterns, Sustainability, 15(21): 15300.
https://doi.org/10.3390/su152115300
Haberman A., Dag A., Shtern N., Zipori I., Erel R., Ben-Gal A., and Yermiyahu U., 2019, Significance of proper nitrogen fertilization for olive productivity in intensive cultivation, Scientia Horticulturae, 246: 710-717.
https://doi.org/10.1016/j.scienta.2018.11.055
Han Y., Wang G., Wu T., Chen W., Ji Y., and Jin S.H., 2021, Fertilization failed to make positive effects on Torreya grandis in severe N-deposition subtropics, Sustainability, 13(17): 9736.
https://doi.org/10.3390/su13179736
Hu S., Wang C., Zhang R., Gao Y., Li K., and Shen J., 2024, Optimizing pollen germination and subcellular dynamics in pollen tube of Torreya grandis, Plant Science, 348: 112227.
https://doi.org/10.1016/j.plantsci.2024.112227
Jangid R., Kumar A., Masu M.M., Kanade N.M., and Pant D., 2023, Alternate bearing in fruit crops: causes and control measures, Asian Journal of Agricultural and Horticultural Research, 10(1): 10-19.
https://doi.org/10.9734/ajahr/2023/v10i1217
Khezri M., Heerema R., Brar G., and Ferguson L., 2020, Alternate bearing in pistachio (Pistacia vera L.): a review, Trees, 34: 855-868.
https://doi.org/10.1007/s00468-020-01967-y
Krasniqi A.L., Blanke M.M., Kunz A., Damerow L., Lakso A.N., and Meland M., 2017, Alternate bearing in fruit tree crops: past, present and future, Acta Horticulturae, 1177: 241-248.
https://doi.org/10.17660/ActaHortic.2017.1177.35
Lazare S., Zipori I., Cohen Y., Haberman A., Goldshtein E., Ron Y., Rotschild R., and Dag A., 2021, Jojoba pruning: new practices to rejuvenate the plant, improve yield and reduce alternate bearing, Scientia Horticulturae, 277: 109793.
https://doi.org/10.1016/j.scienta.2020.109793
Ma X., Huang D., Huang C., Tong Y., Yuan F., Ma X., Liu H., and Fu S., 2023, The application of nitrogen, phosphorus, and potassium regulate the growth and morphological development of Torreya grandis (Taxaceae) saplings, Horticulturae, 9(11): 1203.
https://doi.org/10.3390/horticulturae9111203
Mesejo C., Martínez-Fuentes A., Reig C., Balasch S., Primo-Millo E., and Agustí M., 2020, Mechanical pruning attenuates alternate bearing in ‘Nadorcott’ mandarin, Scientia Horticulturae, 261: 108993.
https://doi.org/10.1016/j.scienta.2019.108993
Netsawang P., Damerow L., Lammers P.S., Kunz A., and Blanke M., 2023, Alternative approaches to chemical thinning for regulating crop load and alternate bearing in apple, Agronomy, 13(1): 112.
https://doi.org/10.3390/agronomy13010112
Rosecrance R.C., Weinbaum S.A., and Brown P.H., 1998, Alternate bearing affects nitrogen, phosphorus, potassium and starch storage pools in mature pistachio trees, Annals of Botany, 82(4): 463-470.
https://doi.org/10.1006/anbo.1998.0696
Shalom L., Samuels S., Zur N., Shlizerman L., Zemach H., Weissberg M., Ophir R., Blumwald E., and Sadka A., 2012, Alternate bearing in citrus: changes in the expression of flowering control genes and in global gene expression in ON- versus OFF-crop trees, PLoS One, 7(10): e46930.
https://doi.org/10.1371/journal.pone.0046930
Sharma N., Singh S.K., Mahato A.K., Ravishankar H., Dubey A.K., and Singh N.K., 2019, Physiological and molecular basis of alternate bearing in perennial fruit crops, Scientia Horticulturae, 243: 214-225.
https://doi.org/10.1016/j.scienta.2018.08.021
Stander O.P.J., Barry G.H., and Cronjé P.J.R., 2018, Fruit load limits root growth, summer vegetative shoot development, and flowering in alternate-bearing ‘Nadorcott’ mandarin trees, Journal of the American Society for Horticultural Science, 143(3): 213-225.
https://doi.org/10.21273/JASHS04438-18
Tang H., Hu Y.Y., Yu W.W., Song L.L., and Wu J.S., 2015, Growth, photosynthetic and physiological responses of Torreya grandis seedlings to varied light environments, Trees, 29(4): 1011-1022.
https://doi.org/10.1007/s00468-015-1180-9
Weinbaum S.A., Picchioni G.A., Muraoka T.T., Ferguson L., and Brown P.H., 1994, Fertilizer nitrogen and boron uptake, storage, and allocation vary during the alternate-bearing cycle in pistachio trees, Journal of the American Society for Horticultural Science, 119(1): 24-31.
https://doi.org/10.21273/JASHS.119.1.24
Zhang X.L., and Xiao L.Y., 2011, Growth and development rhythm of Torreya grandis fruit, Hunan Forestry Science and Technology, 38(3): 36-38.
Zhang R., Zhang Y., Song L., Song X.Z., Hänninen H., and Wu J., 2017, Biochar enhances nut quality of Torreya grandis and soil fertility under simulated nitrogen deposition, Forest Ecology and Management, 391: 321-329.
https://doi.org/10.1016/j.foreco.2017.02.036
. FPDF(win)
. FPDF(mac)
. HTML
. Online fPDF
Associated material
. Readers' comments
Other articles by authors
. Tiejian He

Related articles
. Torreya grandis
. Alternate bearing
. Crop load
. Tree nutrition
. Stable-yield cultivation
Tools
. Post a comment